Computational Evaluation of Probiotic Peptide Interactions with Pro-Inflammatory cytokine Receptors Implicated in Inflammatory Bowel Disease
 , Pentyala Akhil Surya, Puru Bhavi Teja, , Pennahobulappa gari Jayasimha gari Jahnavi and Ghangiri Venkataramanappa Gari Parameswar
Department of Pharmacology, Raghavendra Institute of Pharmaceutical Education and Research, Jawaharlal Nehru Technological University Anantapur, K R Palli Cross, Andhra Pradesh, India
Corresponding Author E-mail: praveenpharmaco@gmail.com
Download this article as:
ABSTRACT:Probiotic-derived peptides have emerged as promising immunomodulatory agents capable of regulating cytokine-mediated inflammatory responses. Interleukin signaling pathways involving IL-4α, IL-21, and IL-23 play a central role in the pathogenesis of inflammatory bowel disease (IBD), particularly ulcerative colitis. This study aimed to evaluate the molecular interactions and binding stability of Lactobacillus-derived probiotic peptides—Surface layer protein A (Slp A), Plantaricin JK (Pln JK), and Plantaricin EF (Pln EF)—with key pro-inflammatory interleukin receptors using in silico approaches. Protein–protein docking was performed using HDOCK, followed by binding free energy estimation via HawkDock and structural interaction visualization using PyMOL. Docking scores, binding free energies, RMSD values, and hydrogen bonding interactions were analyzed to assess binding affinity, stability, and interaction specificity. Slp A demonstrated the strongest interaction with IL-21R C, exhibiting the lowest docking score (−276.84) and highly favorable binding free energy (−88.65 kcal/mol), indicating strong predicted complex stability. Significant interactions were also observed with IL-23 receptor subunits. Pln JK showed selective and stable binding toward IL-23 receptor B and C chains, supported by highly favorable docking scores (−287.76 to −293.17) and low RMSD values, suggesting conformational stability. Pln EF exhibited robust binding with IL-21R C and IL-23R C, reflected by strong docking scores (−241.99 to −291.38) and negative binding free energies (up to −67.74 kcal/mol). Hydrogen bond analysis revealed consistent residue-level interactions across complexes, reinforcing binding specificity. The integrated docking and binding energy analyses highlight Slp A, Pln JK, and Pln EF as promising probiotic peptides with potential receptor interaction requiring biological validation against IL-4α, IL-21, and IL-23 signaling pathways. These findings support their therapeutic relevance in modulating pro-inflammatory responses in IBD and warrant further experimental and structural validation.
KEYWORDS:Antimicrobial Peptides; Binding Free Energy; Cytokines; Molecular Docking Simulation; Ulcerative Colitis
Introduction
Ulcerative colitis (UC) is a chronic relapsing inflammatory disorder of the colon characterized by a dysregulated mucosal immune response, in which pro‑inflammatory cytokine networks play a central pathogenic role.1 Elevated expression and signaling of cytokines such as interleukin-4α (IL-4Rα), interleukin‑21 (IL‑21R) and interleukin‑23 (IL‑23R), and their receptors, amplify T‑cell–driven inflammation, promote Th1/Th17 skewing, and contribute to epithelial barrier dysfunction and sustained mucosal damage in UC.2 In particular, the IL‑23/IL‑23R axis is recognized as a key conductor of innate and adaptive immune responses in the intestinal mucosa, and genetic as well as functional data highlight IL‑23R as a promising therapeutic target in inflammatory bowel disease, including UC.3
Probiotics and their secreted antimicrobial peptides (bacteriocins) and anti‑inflammatory peptides have emerged as attractive candidates to restore intestinal homeostasis by modulating gut microbiota composition, dampening pro‑inflammatory signaling, and reinforcing epithelial barrier function.4 These probiotic‑derived peptides can directly exert antimicrobial effects against pathogenic bacteria, interfere with pathogen adhesion, and attenuate inflammatory cascades by targeting host or microbial factors involved in cytokine production and immune cell activation.5 Recent in silico and in vitro studies suggest that such peptides may interact with key immune receptors and signaling proteins relevant to colorectal inflammation, supporting the rationale to explore their binding to UC‑associated cytokine receptors at atomic resolution.6
In silico protein‑protein docking offers a cost‑effective and mechanistically informative framework to predict the binding modes, affinities and interfacial determinants governing peptide–receptor recognition.7 Structure‑based docking combined with rigorous structure preparation and binding site identification enables systematic evaluation of how probiotic antimicrobial and anti‑inflammatory peptides might engage the extracellular domains of IL‑4Rα, IL‑21R and IL‑23R implicated in UC pathogenesis.8 The HDOCK server provides an integrated, hybrid template‑based and ab initio docking platform for modeling protein–protein complexes, allowing for global search of plausible binding poses followed by scoring and ranking according to shape and physicochemical complementarity.9
To increase the reliability of docking‑derived models, post‑docking free‑energy–based re‑scoring and rigorous interface analysis are essential.10 HawkDock combines docking with molecular mechanics/generalized Born surface area (MM/GBSA) calculations to estimate binding free energy and identify key energetic hot‑spot residues, providing an improved assessment of complex stability compared with docking scores alone.11 Updated implementations of HawkDock incorporate enhanced MM/GBSA variants and deep‑learning–assisted docking to better handle protein–protein interfaces, particularly for charged and flexible complexes, which are common features of cytokine–receptor interactions.12 Complementary visualization and annotation using PDBsum deliver detailed pictorial summaries of secondary structure organization, domain architecture and non‑covalent contacts at the peptide–receptor interface, thereby facilitating structural interpretation of in silico findings and their integration with immunological knowledge of UC.13
Within this methodological framework, the present in silico study systematically interrogates the binding mechanisms between probiotic antimicrobial, anti‑inflammatory peptides.14 UC‑relevant pro‑inflammatory cytokine receptors, with the overarching aim of identifying candidate peptide–receptor interactions that may underlie, or be harnessed for, novel therapeutic strategies in ulcerative colitis.15
Materials and Methods
Structure Retrieval
The molecular details of pro-inflammatory cytokine receptors and antimicrobial-anti-inflammatory peptides are retrieved from Research Collaboratory for Structural Bioinformatics Protein Data Bank (RCSB PDB) having PDB id: IL‑4Rα (1IAR:B), IL‑21R (3TGX:A/B), IL‑23R (5MZV:A/B/C), Slp‑A (7QFG:A), Pln‑JK (2KHF:chains for PlnK/PlnJ), Pln‑EF (2RLW:Pln E/PlnF). With selected length of 336 AA (IL-4Rα), 353AA (IL-21R), 1,012AA (IL-23R) and 149AA (Slp-A), 25AA (Pln-JK), 34AA (Pln-EF). Where resolution 2.30Aº (IL-4Rα), 2.80Aº (IL-21R), 2.80Aº (IL-23R) and1.65Aº (Slp-A) are extracted from X-ray diffraction method and 2KHF (Pln-JK), 2RLW (Pln-EF) extracted with Solution NMR was retrieved from the Research Collaboratory for Structural Bioinformatics Protein Data Bank (RCSB-PDB).
Structure preparation and binding sites identification
Structure preparation is a crucial initial step in protein-protein docking studies to ensure accurate and reliable results. Using BIOVIA Discovery Studio, the protein structure is first imported, and any waters were selectively retained if within 5 Å of the active site others removed. Glycosylation on residues was removed as non-essential and to clean the structure. Missing residues and atoms are added, and hydrogen atoms are assigned appropriately to reflect physiological conditions. The structure is then optimized through energy minimization by applying field force like CHARMm force field to relieve any steric clashes while maintaining the protein’s overall conformation. Once prepared, the protein is saved for subsequent docking analysis. For binding pocket prediction, tools such as ProteinPlus and Anchor Studio are employed to identify potential protein interaction sites. Binding site guided docking is then performed using these predicted pockets. Protein Plus uses structural features and geometric algorithms to locate cavities and grooves on the protein surface that are likely binding pockets. Anchor Studio further refines this prediction by analysing binding hot spots, allowing for precise mapping of interaction sites relevant for docking.
Molecular docking of pro-inflammatory protein (IL-4Rα), (IL-21R), (IL-23R) to anti-inflammatory peptide (Slp-A) and anti-microbial peptides
The molecular docking using HDOCK a series of well-defined steps to predict how two proteins interact at molecular level. The prepared proteins were uploaded to the HDOCK server alongside flexible ligands. HDOCK employs a hybrid docking algorithm combining template-based modeling with FFT-based rigid-body docking, where the receptor remains fixed while the ligand explores conformational flexibility to find the best binding models. User can specify binding sites if known or allow for blind docking for unbiased prediction. HDOCK generates multiple docked poses ranked by scoring functions that estimate binding affinity and interaction quality. The top-ranked complexes are further analyzed for interaction details, and validation metrics such as root mean square deviation (RMSD) and interface analysis are used to assess the docking accuracy.
Docking validation
Docking validation was performed by calculating the Root Mean Square Deviation (RMSD) of the top HDOCK pose against the crystal structure from PDB using PyMOL (RMSD threshold for success). Binding free energy was further validated using HawkDock’s MM/GBSA method.
Validation of docking results is a critical step to ensure that the predicted protein-protein interactions are accurate and biologically meaningful. The Root Mean Square Deviation (RMSD) score is commonly used for this purpose and can be calculated using PyMOL software. RMSD to measure the average distance between atoms of the docked protein–ligand complex.16 A lower RMSD value indicates a close match between the predicted and reference structures, suggesting that the docking pose is reliable. In addition to RMSD, binding free energy calculation is an important validation metric that reflects the stability and strength of the interaction between proteins. HawkDock is a computational tool that predicts the binding free energy by combining docking results with molecular mechanics and solvation models. A more negative binding free energy indicates a stronger and more stable protein-protein interaction.
Analysis and visualization
Generalized Born surface area (MM/GBSA) analysis was conducted using HawkDock to estimate the binding free energy of protein-protein complexes. HawkDock integrates docking results with molecular mechanics energy calculations and solvation models to provide an accurate and reliable estimation of interaction stability. The MM/GBSA approach decomposes the total binding free energy into contributions from van der Waals, electrostatic, polar solvation, and nonpolar solvation energies, allowing detailed insight into the forces stabilizing the complex. This method offers improved accuracy over docking scores alone and serves as an essential step to validate the predicted interactions.
Visualization of protein structures and interactions using PDBsum is an important step to present comprehensive and clear structural insights in a docking study. PDBsum is a well-recognized pictorial database that summarizes 3D protein structures deposited in the Protein Data Bank (PDB). It automatically provides multiple schematic diagrams such as secondary structure elements, protein domains, and intermolecular interactions including protein-protein interfaces. The visual outputs from PDBsum include interactive 3D viewers for the protein complex, showing surface clefts, binding pockets, and interface residues, which are crucial for understanding docking results. PDBsum also generates detailed interaction maps highlighting hydrogen bonds, salt bridges, and hydrophobic contacts that stabilize the complex.
Results
Analysis and validation of docked complexes of probiotic peptides (Slp A), (Pln JK) & (Pln EF) and Pro-inflammatory proteins (IL4α), (IL21) & (IL23)
The docking analyses reveal that Slp A exhibited the most favorable binding with IL-21R C, indicated by the lowest docking score (-276.84) and highest negative binding free energy (-88.65). However, the top pose showed substantial positional deviation (RMSD = 19.194 Å), suggesting score-based ranking favors affinity over precise geometry cluster 2 pose (RMSD <2.0 Å) was prioritized for analysis. IL 23R C also demonstrated significant interaction strength. In contrast, IL 21R B showed weaker affinity with higher RMSD (5.432), reflecting less stability. The trend in binding free energies corresponds closely with docking scores, indicating strong binding affinity for select Slp A–interleukin complexes. Elevated RMSD values for some complexes imply conformational deviations, which may impact functional interaction. Overall, these findings highlight specific Slp A–interleukin interactions with high therapeutic promise for modulating pro-inflammatory responses in IBD, warranting further structural validation. (Table -1). Pln JK exhibited strong interaction with IL 23RC and IL 23R B, as indicated by favorable docking scores (-293.17 and -287.76) and notably low RMSD (2.940 and 0.042), suggesting stable complexes. The highest binding free energy (-63.51) was seen with IL 4R alfa B, supporting robust inhibitory potential. In contrast, IL 21R B and IL 23R D showed modest affinity and stability with less negative binding energies and slightly elevated RMSD values. Overall, the trend across metrics highlights Pln JK’s selective, potentially therapeutic interaction, especially with IL23 subtypes, for downregulating inflammatory response in IBD. Further validation studies are needed to confirm biological efficacy and structural stability. (Table -2). Pln EF demonstrated the strongest interaction with IL 21R C, as evidenced by its considerable docking score (-241.99) and highly negative binding energy (-67.74), suggesting a stable and potentially effective inhibitory complex. Notably, IL 23R C also showed favorable docking metrics (-291.38, -55.12), though RMSD values were elevated, implying possible structural rearrangements post-docking. IL 21R B had lower RMSD (1.372), indicating greater rigidity and structural integrity of the complex. Overall, Pln EF selectively binds to IL21 and IL23 subtypes, supporting its putative role in mitigating pro-inflammatory pathways relevant to IBD. These findings merit further experimental validation to confirm biological efficacy and mechanistic impact on inflammation regulation. (Table -3)
Table 1: Analysis and validation of docked complexes of probiotic peptides (Slp A) and Pro-inflammatory proteins (IL4α, IL21 and IL23).
|
Probiotic protein (Slp A) and Pro-inflammatory proteins. (IL4α), (IL21) & (IL23) |
Docking score by H DOCK | Binding free energy by HAWKDOCK | RMSD by PyMol |
| IL 4R alfa B Slp A | -274.19 | -45.01 |
12.165 |
|
IL 21R B Slp A |
-210.74 | -12.79 | 5.432 |
| IL 21R C Slp A | -276.84 | -88.65 |
9.771 |
|
IL 23R B Slp A |
-225.71 | -56.95 | 9.964 |
| IL 23R C Slp A | -283.78 | -61.25 |
19.194 |
|
IL 23R D Slp A |
-229.41 | -26.73 |
13.377 |
Table 2: Analysis and validation of docked complexes of probiotic peptides (Pln JK) and Pro-inflammatory proteins (IL4α, IL21 and IL23).
|
Probiotic protein (Pln JK) and Pro-inflammatory proteins. (IL4α), (IL21) & (IL23) |
Docking score by H DOCK | Binding free energy by HAWKDOCK | RMSD by PyMol |
| IL 4R alfa B Pln JK | -282.49 | -63.51 |
2.277 |
|
IL 21R B Pln JK |
-224.97 | -44.22 | 1.527 |
| IL 21R C Pln JK | -265.18 | -36.16 |
2.661 |
|
IL 23R B Pln JK |
-287.76 | -51.46 | 0.042 |
| IL 23RC Pln JK | -293.17 | -58.32 |
2.940 |
|
IL 23R D Pln JK |
-250.25 | -43.86 |
5.693 |
Table 3: Analysis and validation of docked complexes of probiotic peptides (Pln EF) and Pro-inflammatory proteins (IL4α, IL21 and IL23).
|
Probiotic protein (Pln EF) and Pro-inflammatory proteins. (IL4α), (IL21) & (IL23) |
Docking score by H DOCK | Binding free energy by HAWKDOCK | RMSD by PyMol |
| IL 4R alfa B Pln EF | -272.85 | -46.02 |
6.228 |
|
IL 21R B Pln EF |
-224.96 | -41.79 | 1.372 |
| IL 21R C Pln EF | -241.99 | -67.74 |
6.329 |
|
IL 23R C Pln EF |
-291.38 | -55.12 | 6.313 |
| IL 23R D Pln EF | -249.06 | -47.67 |
6.394 |
Interaction between probiotic Lactobacillus Surface layer protein A (Slp A protein and IL 4α, IL 21 and IL 23
Molecular docking revealed strong hydrogen bonding interactions between Lactobacillus probiotic Surface layer protein A (Slp A) and Interleukin-4 alpha (IL-4α). Key Slp A residues TYR326, TYR328, ALA332, and LYS358 formed hydrogen bonds with HIS131, THR133, GLN181, and ALA182 of IL-4α, indicating a stable and specific binding interface. The complex exhibited a HDOCK score of −274.18, suggesting highly favorable binding affinity. Furthermore, the HAWK DOCK binding free energy of −12.99 kcal/mol confirmed strong thermodynamic stability. These results demonstrate that Slp A may effectively interact with IL-4α, potentially influencing it’s signalling mechanism and contributing to immunomodulatory effects of Lactobacillus probiotics (Table -4, Fig -A.). The molecular docking analysis revealed strong hydrogen bonding interactions between Lactobacillus probiotic Surface layer protein A (Slp A) residues (ASN 324, ALA 416) and Interleukin 21 B-chain (GLN 3, LEU 123) residues, indicative of stable protein-protein complex formation. The docking score obtained from HDOCK was -210.74, complemented by a binding free energy of -12.79 kcal/mol as predicted by HAWKDOCK, confirming a favorable and energetically stable interaction. These results suggest that Slp A may effectively modulate proinflammatory IL-21 signaling through specific hydrogen bonding interactions, offering potential anti-inflammatory benefits. (Table -4, Fig -B). The docking analysis demonstrated multiple hydrogen bonding interactions between Lactobacillus probiotic Surface Layer Protein A (Slp A) residues (including LYS 358, TYR 328, LYS 333, GLY 357, ARG 384, ARG 444, LYS 425) and Interleukin 21 C-chain residues (LEU 28, SER 47, LEU 48, THR 61, SER 76, GLN 78, GLN 82, SER 87, GLU 89). The highly negative docking score of -276.84 (HDOCK) and strong binding free energy of -88.65 kcal/mol (HAWKDOCK) indicate robust and energetically favourable protein-protein interactions. These findings suggest Slp A forms stable complexes with IL-21 C-chain, supporting its potential as an effective anti-inflammatory agent. (Table -4, Fig -C). The hydrogen bonding interactions between Lactobacillus probiotic Surface Layer Protein A (Slp A) residues (Asn422, Tyr391, Leu445, Lys439) and Interleukin 23 (IL-23) B-chain residues (Thr42, Cys77, Arg167, Ala174) indicate a stable and specific protein-protein complex. The HDOCK docking score of -225.71 and binding free energy of -56.95 kcal/mol by HAWKDOCK reflect strong binding affinity and energetic favourability for this interaction. These findings suggest Slp A may have significant potential in modulating IL-23 mediated inflammatory signaling, supporting its possible therapeutic application in inflammation-related disorders. (Table -4, Fig -D). Docking studies revealed extensive hydrogen bonding interactions between Lactobacillus probiotic Surface Layer Protein A (Slp A) residues (Thr353, Thr354, Thr385, Asn351, Thr352, Arg444, Lys425, Thr419, His323, Ser417) and Interleukin 23 (IL-23) C-chain residues (Glu130, Tyr138, Gly149, Tyr178, Ala222, Val224, Ile225, Asp243, Ser309). The highly negative HDOCK docking score of -283.78 and binding free energy of -61.25 kcal/mol by HAWKDOCK indicate a strong, stable, and energetically favourable complex. These findings support Slp A’s potential in modulating IL-23 driven inflammation, highlighting its therapeutic relevance against inflammatory diseases. (Table -4, Fig -E). The docking study revealed hydrogen bonding interactions between Lactobacillus probiotic Surface Layer Protein A (Slp A) residues (Tyr326, Lys421, Gly336, Arg334, Thr419) and Interleukin 23 (IL-23) D-chain residues (Trp31, Glu44, Arg52, Phe102, Ser108, Asp111). The HDOCK docking score of -229.41 and binding free energy of -26.73 kcal/mol (HAWKDOCK) demonstrate a strong, energetically favourable protein-protein association. These interactions support the potential of Slp A to modulate IL-23 D-chain mediated inflammatory pathways, indicating its promise as an anti-inflammatory therapeutic candidate. Such binding may attenuate pro-inflammatory signaling in immune responses. (Table -4, Fig -F).
Table 4: Hydrogen bonding interaction between residues of Surface layer protein A (Slp A) and (IL4α, IL21 and IL23).
|
Lactobacillus Surface layer protein A (Slp A) residues |
Interleukin
4 α (IL 4α) residues |
Interleukin 21 (IL 21) residues |
Interleukin 23 B-chain (IL 23) residues |
|
TYR 326 |
HIS 131, GLN 181, THR 133 | ||
|
ALA 332 |
HIS 131 | ||
| THR 419 |
AGR 177 |
||
|
TYR 328 |
ALA 182 | SER 47 | |
| LYS 358 | ALA 182 |
LEU 28, LEU 48 |
|
|
LYS 425 |
THR 186 | Asp243 | |
| THR 419 | TRP 187 |
Ile225, SER 108, ASP 111 |
|
|
ASN 324 |
GLN 3 | ||
| ALA 416 |
LEU 123 |
||
|
LYS 333 |
THR 61 | ||
| LYS 425 |
SER 76 |
||
|
TYR 427 |
GLN 78 | ||
| GLY 357 |
GLN 82 |
||
|
ARG 384 |
SER 87 | ||
| ARG 444 |
SER 87 |
||
|
LYS 425 |
GLU 89 | ||
| Asn422 |
Thr42 |
||
|
Tyr391 |
Cys77 | ||
| Leu445 |
Arg167 |
||
|
Lys439 |
Ala174 | ||
| Thr353 |
Glu130 |
||
|
Thr354 |
Glu130 | ||
| Thr385 |
Tyr138 |
||
|
Asn351 |
Gly149 | ||
| Arg444 |
Ala222 |
||
|
Lys425 |
Val224 | ||
| His323 |
Ser309 |
||
|
Ser417 |
Ser309 | ||
| Lys421 |
Glu44 |
||
|
Gly336 |
Arg52 | ||
| Arg334 |
Phe102 |
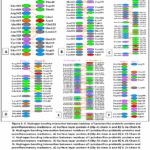 |
Figure 1: A: Hydrogen bonding interaction between residues of Lactobacillus probiotic proteins and proinflammatory mediators. A) Surface layer protein A (Slp A) chain A and B) IL 4α Chain B.; B: Hydrogen bonding interaction between residues of Lactobacillus probiotic proteins and proinflammatory mediators. A) Surface layer protein A (Slp A) chain A and B) IL 21 Chain B. |
Interaction between probiotic Lactobacillus probiotic Plantercin JK protein and IL 4α, IL 21 and IL 23
Hydrogen bonding analysis indicated a strong and specific interaction between Lactobacillus probiotic Plantercin JK (Pln JK) residue ALA 22 and Interleukin 4 alpha (IL-4α) residue ARG 175. The HDOCK docking score of -282.49, along with a binding free energy of -63.51 kcal/mol by HAWKDOCK, highlights a highly stable and energetically favorable complex formation. These interaction metrics suggest that Pln JK may effectively bind to and regulate IL-4α–mediated proinflammatory signaling, providing valuable evidence for its therapeutic potential in immune and inflammatory conditions through robust hydrogen bond formation. (Table -5, Fig -G). The docking study showed strong hydrogen bonding interactions between Lactobacillus probiotic Plantercin JK (Pln JK) residues (ARG 11, TYR 15) and Interleukin 21 (IL-21) B-chain residues (THR 40, ASN 41, GLU 43, THR 81). The HDOCK docking score of -224.97 and binding free energy of -44.32 kcal/mol by HAWKDOCK reflect a stable and energetically favorable interaction. These specific hydrogen bonds suggest that Pln JK may effectively modulate IL-21-mediated proinflammatory processes, supporting its therapeutic potential as an anti-inflammatory agent by stabilizing interactions with key cytokine residues. (Table -5, Fig -H). Hydrogen bonding analysis showed that Lactobacillus probiotic Plantercin JK (Pln JK) residues (ALA 19, TYR 15) formed stable interactions with Interleukin 21 (IL-21) C-chain residues (GLN 140, SER 151). The highly negative HDOCK docking score of -265.18 and binding free energy of -36.16 kcal/mol by HAWKDOCK confirm strong and favorable protein-protein binding. These findings indicate that Pln JK can potentially modulate IL-21 C-chain-mediated inflammatory pathways via robust hydrogen bonding, supporting its role as a promising anti-inflammatory therapeutic agent. (Table -5, Fig -I). Hydrogen bonding analysis revealed strong interactions between Lactobacillus probiotic Plantercin JK (Pln JK) residues (ARG 11, ILE 23) and Interleukin 23 (IL-23) B-chain residues (ALA 47, ARG 178). The HDOCK docking score of -287.76 and binding free energy of -51.46 kcal/mol (HAWKDOCK) confirm highly stable and energetically favorable binding. These data suggest that Pln JK forms robust hydrogen bonds with key IL-23 B-chain residues, supporting its efficacy as an anti-inflammatory agent by potentially modulating IL-23–driven inflammatory pathways through strong and specific molecular recognition. (Table -5, Fig -J). Hydrogen bonding analysis demonstrated robust interactions between Lactobacillus probiotic Plantercin JK (Pln JK) residues (ARG 25, TYR 15, TRP 7) and Interleukin 23 (IL-23) C-chain residues (GLU 130, GLN 305, PRO 306, SER 309). The very strong HDOCK docking score of -293.17 and binding free energy of -58.32 kcal/mol (HAWKDOCK) indicate highly stable and energetically favorable binding. These results highlight the strong potential of Pln JK in targeting IL-23 C-chain, suggesting functional inhibition of inflammatory pathways via specific and stable hydrogen bond formation, supporting its value as an anti-inflammatory agent. (Table -5, Fig -K). The docking analysis showed strong hydrogen bonding interactions between Lactobacillus probiotic Plantercin JK (Pln JK) residues (ARG 25, ALA 19, ARG 11) and Interleukin 23 (IL-23) D-chain residues (GLN 39, ARG 45, ASP 111). With a highly favorable HDOCK docking score of -250.25 and a binding free energy of -43.86 kcal/mol by HAWKDOCK, the results suggest a stable and energetically robust complex. These findings support the anti-inflammatory potential of Pln JK, indicating it may effectively inhibit IL-23 D-chain proinflammatory actions via multiple strong hydrogen bond interactions. (Table -5, Fig -L).
Table 5: Hydrogen bonding interaction between residues of Plantercin JK (Pln-JK) and (IL4α, IL21 and IL23).
|
Lactobacillus probiotic Plantercin JK (Pln JK) residues |
Interleukin 4α (IL 4α) residues | Interleukin 21 B-chain (IL 21) residues |
Interleukin 23 (IL 23) residues |
|
ALA 22 |
ARG 175 | ||
| ARG 11 | THR 40, ASN 41 |
ALA 47, ASP 111 |
|
|
TYR 15 |
GLU 43, THR81 | ||
| ALA 19 |
GLN 140 |
||
|
TYR 15 |
SER 151 | GLN 305, PRO 306 | |
| ILE 23 |
ARG 178 |
||
|
ARG 25 |
GLU 130 | ||
| TRP 7 |
SER 309 |
||
|
ARG 25 |
GLN 39 | ||
| ALA 19 |
ARG 45 |
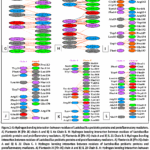 |
Figure 2: G: Hydrogen bonding interaction between residues of Lactobacillus probiotic proteins and proinflammatory mediators. A) Plantercin JK (Pln JK) chain A and B) IL 4α Chain B. H: Hydrogen bonding interaction between residues of Lactobacillus probiotic proteins and proinflammatory mediators. A) Plantercin JK (Pln JK) chain A and B) IL 21 Chain B. |
Interaction between probiotic Lactobacillus probiotic Plantercin EF protein and IL 4α, IL 21 and IL 23
The docking analysis identified strong hydrogen bonding interactions between Lactobacillus probiotic Plantercin EF (Pln EF) residues (TYR 5, VAL 1, SER 6, ASN 13) and Interleukin 4 alpha (IL-4α) residues (ASN 130, TYR 154, GLN 181, TRP 187). The HDOCK docking score of -272.85 and binding free energy of -46.02 kcal/mol by HAWKDOCK indicate a stable and energetically favorable complex. These results suggest Pln EF has potential as an anti-inflammatory agent by effectively interfacing with IL-4α and possibly inhibiting its proinflammatory activity through robust hydrogen bonding. (Table -6, Fig -M). Docking studies demonstrated hydrogen bonding interactions between Lactobacillus probiotic Plantercin EF residues (TYR 5, VAL 10, PHE 2) and Interleukin 21 (IL-21) B-chain residues (ARG 5, LYS 73, SER 80). The HDOCK docking score of -224.96 and binding free energy of -41.79 kcal/mol by HAWKDOCK highlight a stable and energetically favorable complex. These results indicate the potential of Pln EF to interfere with IL-21 B-chain’s proinflammatory signaling through specific hydrogen bonding, supporting its inhibitory efficacy as an anti-inflammatory agent. (Table -6, Fig -N). Hydrogen bonding analysis indicated that Lactobacillus probiotic Plantercin EF residues (VAL 1, ASP 22) form strong and multiple hydrogen bond interactions with Interleukin 21 (IL-21) C-chain residues (SER 92, ARG 142, ARG 154). The highly negative HDOCK docking score of -241.99 and binding free energy of -67.74 kcal/mol by HAWKDOCK suggest an exceptionally stable and energetically favorable protein-protein complex. This supports the potential of Plantercin EF as an anti-inflammatory agent, capable of modulating IL-21 C-chain–driven immunological responses by robust binding at key residues, thus targeting proinflammatory pathways effectively. (Table -6, Fig -O). Hydrogen bonding analysis indicated multiple strong interactions between Lactobacillus probiotic Plantercin EF (Pln EF) residues (Tyr5, Asn13, Arg11) and Interleukin 23 (IL-23) C-chain residues (Ser221, Arg295, Thr145, Glu130, Thr132). The HDOCK docking score of -291.38 and binding free energy of -55.12 kcal/mol by HAWKDOCK confirm a highly stable and energetically favorable complex. This suggests Pln EF can effectively interact with and inhibit IL-23 C-chain–mediated proinflammatory pathways by forming robust hydrogen bonds, supporting its significance as a potential anti-inflammatory and immunomodulatory therapeutic agent. (Table -6, Fig -P). Hydrogen bonding analysis revealed strong interactions between Lactobacillus probiotic Plantercin EF (Pln EF) residues (Tyr5, Val10, Val24, Ile25, Val1) and Interleukin 23 (IL-23) D-chain residues (Gln39, Arg45, Ser100, Asp111, Gln118, Thr120). The HDOCK docking score of -249.06 and binding free energy of -47.67 kcal/mol by HAWKDOCK indicate stable and energetically favorable protein-protein association. These observations suggest that Pln EF may effectively inhibit IL-23 D-chain mediated proinflammatory activity by robust hydrogen bonding interactions, reinforcing its anti-inflammatory and immunomodulatory potential. (Table -6, Fig -Q).
Table 6: Hydrogen bonding interaction between residues of Plantercin EF (Pln-EF) and (IL4α, IL21 and IL23).
|
Lactobacillus probiotic Plantercin EF (Pln EF) residues |
Interleukin 4 alfa (IL 4α) residues | Interleukin 21 residues |
Interleukin 23 (IL23) residues |
|
TYR 5 |
ASN 130 | ARG 5 | SER 221,
GLN 39 |
| VAL 1 | TYR 154 | SER 92 |
GLN 118, THR 120 |
|
SER 6 |
GLN 181 | ||
|
ASN 13 |
TRP 187 |
||
| VAL 10 | LYS 73 |
ARG 45 |
|
|
PHE 2 |
SER 80 | ||
| ASP 22 |
ARG 142, ARG 154 |
||
|
Asn13 |
ARG 295 | ||
| ARG11 |
THR 145, GLU 130, THR 132 |
||
|
Ile25 |
Ser100 | ||
| Val24 |
Asp111 |
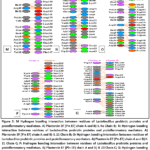 |
Figure 3: M: Hydrogen bonding interaction between residues of Lactobacillus probiotic proteins and proinflammatory mediators. A) Plantercin EF (Pln EF) chain A and B) IL 4α Chain B; N: Hydrogen bonding interaction between residues of Lactobacillus probiotic proteins and proinflammatory mediators. A) Plantercin EF (Pln EF) chain A and B) IL 21 Chain B |
Discussion
Peptides obtained from probiotics are gained attention as bioactive substances capable of altering the host immune response, which goes beyond the commonly known impact of gut microbiota.17 Recent research reveals that particular surface and secreted proteins originating from probiotics possess the capability to directly interact with immune receptors in the host and influence cytokine signalling pathways.18,19 This study presents a comprehensive computational approach that was employed to investigate how Lactobacillus-derived peptides, specifically Slp A, Plantarcin JK (Pln JK), and Plantarcin EF (Pln EF), might impact the immune system concerning essential pro-inflammatory interleukin receptors involved in inflammatory bowel disease (IBD), namely ulcerative colitis.20,21
Interleukins IL-4, IL-21, and IL-23 play a vital role in determining the specialization of immune cells.22 The advancement of inflammatory processes in the pathogenesis of IBD. IL-23 is necessary for the support and proliferation of pathogenic Th 17 cells, whereas IL-21 amplifies immune activation and fosters chronic intestinal inflammation.23 While IL-4 is typically associated with Th2 responses, research has demonstrated that IL-4α signaling leads to an imbalance in mucosal immunity and persistent disease in IBD.24 Consequently, targeting these cytokine pathways with treatment is a logical approach. Among the investigate peptides, Slp A displayed the most powerful and consistent binding affinity, especially for C-chain of the IL-21 receptor.25 The highly favourable docking score (-276.84) and markedly negative binding free energy (-88.65 kcal/mol) signify a stable and exceptionally energetic complex.26
Numerous hydrogen bonding interactions further validate the high specificity of this interaction.27 These findings correspond with prior studies that have indicated that Lactobacillus surface layer proteins are capable of directly binding to immune receptors and modulating cytokine responses at the intestinal level.28 Given the established function of IL-21 in promoting inflammatory responses in IBD, strong Slp A–IL-21R interactions suggest a possible mechanism for mitigation inflammation mediated by IL-21.29 Slp A also exhibited considerable binding affinity for the IL-23 receptor subunits, specifically the C-chain. IL-23–mediated signaling is crucial form maintaining chronic intestinal inflammation through the survival of Th17 cells.30 Thus, Slp A’s capacity to stably interact with IL-23 receptor domains implies its potential therapeutic relevance.31 The elevated RMSD values observed in certain Slp A complexes might be attributed to conformational flexibility rather than instability, which is frequently seen in biologically significant protein–protein interactions.32
Plantaricin JK exhibited selective but highly stable binding, notably with the B and C chains of the IL-23 receptor.33 The remarkably low RMSD values recorded for these complexes indicate minimal conformational change upon binding, suggests potent and durable molecular interactions.34 Elevated docking scores and positive biding free energies further reinforce its inhibitory potential.35 Given that IL-23- targeting biologics have shown success in clinical IBD management, these results imply that Pln JK might offer a peptide-based alternative capable of selectively modulating IL-23 signaling Pln JK also displayed a powerful connection with IL-4α, as evidenced by extremely low binding free energy numbers.36 While IL-4 is not usually thought of as a main cause of IBD, changes in IL-4α signaling have been linked to immune system problems in long term intestinal swelling.37 Because of its specific way of binding, Pln JK could help keep the immune system steady while reducing unwanted immune system suppression.38 Plantaricin EF also exhibited a strong and specific attraction, especially to IL-21R C and IL-23R C. Very good binding free energies and consistent hydrogen bonding patterns point to steady interactions between proteins.39 It is worth noting that lower RMSD valuesin some PlnEF combinations suggest stronger structural firmness and ongoing receptor participation.40 Past research has emphasized how plantaricins fight germs and control the immune system; the current results build on this understanding by giving us a close-up look at how they target cytokine receptors.41
The agreement between docking results, binding free energies, RMSD values,and hydrogen bond studies makes the computational predictions more trustworthy.42 Using confirmed docking platforms like HDOCK and HawkDock gives more weight to the strength of the interaction study.43 Even though computer-based findings cannot completely copy how complex immune responses work in living things, they offer helpful early information for spotting possible therapeutic contenders and guiding experimental confirmation.44
Conclusion
Additionally, experimental confirmation through cytokine blocking tests in test tubes and IBD models in living things will be crucial to verifying how well they work biologically and how safe they are for treatment. However, this research provides a solid computational base that supports the possibility of probiotic peptides derived from Lactobacillus as regulators of IL-4α, IL-21, and IL-23 signaling pathways in inflammatory bowel disease.
This research provides a thorough computational investigation of Surface layer protein A (Slp A), Plantaricin JK (Pln JK), and Plantaricin EF (Pln EF), which are probiotic peptides originating from Lactobacillus, to assess their capacity to influence pro-inflammatory interleukin signaling relevant to inflammatory bowel disease. Through molecular docking, assessment of binding free energy, and examination of structural interactions, it was shown that these peptides bind selectively and with favorable energy to IL-4α, IL-21, and IL-23 receptor components. Notably, Slp A displayed the most substantial and dependable interactions, especially with the IL-21 receptor C-chain, pointing towards significant binding stability and selectivity. Plantaricin JK exhibited selective and consistent interactions with IL-23 receptor variants, whereas Plantaricin EF demonstrated strong binding affinity for both IL-21R C and IL-23R C. The coherence observed across docking scores, binding energies, RMSD values, and hydrogen bonding patterns validates the dependability of the computational forecasts. Collectively, these results emphasize the potential of probiotic derived peptidesas encouraging immunomodulatory agents and establish a robust computational basis for upcomig experimental confirmation and therapeutic advancements in the context of inflammatory bowel disease.
Acknowledgement
The author would like to thank the College of Raghavendra Institute of Pharmaceutical Education and Research for their support of this work.
Funding Sources
The author(s) received no financial support for the research, authorship, and/or publication of this article.
Conflict of Interest
The author(s) do not have any conflicts of interest.
Data Availability Statement
This statement does not apply to this article.
Ethics Statement
This research did not involve human participants, animal subjects, or any material that would require ethical approval.
Informed Consent Statement
This study did not involve human participants; therefore, informed consent was not needed.
Clinical Trial Registration
This research does not involve any clinical trials.
Permission to reproduce material from other sources:
Not applicable
Authors’ contributions
- Pasala Praveen Kumar: Designed the project.
- Pentyala Akhil Surya: Performed the project, carried out docking studies, Literature review, Wrote the paper, collected data.
- Patil Navya Sree: Collected data related to the project and Literature review
- Pennahobulappa gari Jayasimha gari Jahnavi: Literature Review
- Ghanagiri venkataramanappa gar parameswar: Analysis and review.
References
- Tang X, Huang Y, Zhu Y, Xu Y. Immune dysregulation in ulcerative colitis: pathogenic mechanisms and therapeutic strategies of traditional Chinese medicine. Front Cell Dev Biol. 2025;13:1610435. doi:10.3389/fcell.2025.1610435
CrossRef - Woś I, Tabarkiewicz J. Effect of interleukin-6, -17, -21, -22, and -23 and STAT3 on signal transduction pathways and their inhibition in autoimmune arthritis. Immunol Res. 2021;69(1):26-42. doi:10.1007/s12026-021-09173-9
CrossRef - Korta A, Kula J, Gomułka K. The Role of IL-23 in the Pathogenesis and Therapy of Inflammatory Bowel Disease. Int J Mol Sci. 2023;24(12):10172. doi:10.3390/ijms241210172
CrossRef - Gou HZ, Zhang YL, Ren LF, Li ZJ, Zhang L. How do intestinal probiotics restore the intestinal barrier? Front Microbiol. 2022;13:929346. doi:10.3389/fmicb.2022.929346
CrossRef - Barzegari A, Kheyrolahzadeh K, Hosseiniyan Khatibi SM, Sharifi S, Memar MY, Zununi Vahed S. The Battle of Probiotics and Their Derivatives Against Biofilms. Infect Drug Resist. 2020;Volume 13:659-672. doi:10.2147/IDR.S232982
CrossRef - Qiu W, Wang Z, Liu Q, et al. Structure and regulatory mechanisms of food‐derived peptides in inflammatory bowel disease: A review. Food Sci Nutr. 2024;12(9):6055-6069. doi:10.1002/fsn3.4228
CrossRef - Hashemi ZS, Zarei M, Fath MK, et al. In silico Approaches for the Design and Optimization of Interfering Peptides Against Protein–Protein Interactions. Front Mol Biosci. 2021;8:669431. doi:10.3389/fmolb.2021.669431
CrossRef - Nicola G, Abagyan R. Structure‐Based Approaches to Antibiotic Drug Discovery. Curr Protoc Microbiol. 2009;12(1). doi:10.1002/9780471729259.mc1702s12
CrossRef - Li H, Huang E, Zhang Y, Huang S, Xiao Y. HDOCK update for modeling protein‐ RNA / DNA complex structures. Protein Sci. 2022;31(11):e4441. doi:10.1002/pro.4441
CrossRef - Rastelli G, Pinzi L. Refinement and Rescoring of Virtual Screening Results. Front Chem. 2019;7:498. doi:10.3389/fchem.2019.00498
CrossRef - Weng G, Wang E, Wang Z, et al. HawkDock: a web server to predict and analyze the protein–protein complex based on computational docking and MM/GBSA. Nucleic Acids Res. 2019;47(W1):W322-W330. doi:10.1093/nar/gkz397
CrossRef - Zhang X, Jiang L, Weng G, et al. HawkDock version 2: an updated web server to predict and analyze the structures of protein–protein complexes. Nucleic Acids Res. 2025;53(W1):W306-W315. doi:10.1093/nar/gkaf379
CrossRef - Laskowski RA, Jabłońska J, Pravda L, Vařeková RS, Thornton JM. PDBsum: Structural summaries of PDB entries. Protein Sci. 2018;27(1):129-134. doi:10.1002/pro.3289
CrossRef - Arakal BS, Whitworth DE, James PE, et al. In Silico and In Vitro Analyses Reveal Promising Antimicrobial Peptides from Myxobacteria. Probiotics Antimicrob Proteins. 2023;15(1):202-214. doi:10.1007/s12602-022-10036-4
CrossRef - Műzes G. Changes of the cytokine profile in inflammatory bowel diseases. World J Gastroenterol. 2012;18(41):5848. doi:10.3748/wjg.v18.i41.5848
CrossRef - Bachannagari N, Koteswara Rao GSN, Kella A, et al. In Silico and In Vivo Approaches to Evaluate the Cardioprotective Potential of Citronellal by Targeting HMG-CoA Reductase. J Comput Biophys Chem. 2026;25(11):1753-1769. doi:10.1142/S2737416525501145
CrossRef - Romero-Luna HE, Hernández-Mendoza A, González-Córdova AF, Peredo-Lovillo A. Bioactive peptides produced by engineered probiotics and other food-grade bacteria: A review. Food Chem X. 2022;13:100196. doi:10.1016/j.fochx.2021.100196
CrossRef - Vijayaram S, K.E V, Kandasamy S, et al. Probiotics: A multifaceted approach to health promotion-from disease prevention to food enrichment and delivery systems. AIMS Microbiol. 2025;11(3):602-648. doi:10.3934/microbiol.2025026
CrossRef - Guo N, Lv L. Mechanistic insights into the role of probiotics in modulating immune cells in ulcerative colitis. Immun Inflamm Dis. 2023;11(10):e1045. doi:10.1002/iid3.1045
CrossRef - Moll GN, Van Den Akker E, Hauge HH, et al. Complementary and Overlapping Selectivity of the Two-Peptide Bacteriocins Plantaricin EF and JK. J Bacteriol. 1999;181(16):4848-4852. doi:10.1128/JB.181.16.4848-4852.1999
CrossRef - Ma Y, Hu C, Zhang J, et al. Lactobacillus plantarum 69-2 combined with α-lactalbumin hydrolysate alleviates DSS-induced ulcerative colitis through the TLR4/NF-κB inflammatory pathway and the gut microbiota in mice. Food Funct. 2024;15(22):10987-11004. doi:10.1039/D4FO02975E
CrossRef - Keegan AD, Leonard WJ, Zhu J. Recent advances in understanding the role of IL-4 signaling. Fac Rev. 2021;10. doi:10.12703/r/10-71
CrossRef - Liu ZJ, Yadav PK, Su JL, Wang JS, Fei K. Potential role of Th17 cells in the pathogenesis ofinflammatory bowel disease. World J Gastroenterol. 2009;15(46):5784. doi:10.3748/wjg.15.5784
CrossRef - Hoving JC, Keeton R, Höft MA, Ozturk M, Otieno-Odhiambo P, Brombacher F. IL-4 Receptor-Alpha Signalling of Intestinal Epithelial Cells, Smooth Muscle Cells, and Macrophages Plays a Redundant Role in Oxazolone Colitis. Mediators Inflamm. 2020;2020:1-11. doi:10.1155/2020/4361043
CrossRef - Kang L, Bondensgaard K, Li T, Hartmann R, Hjorth SA. Rational Design of Interleukin-21 Antagonist through Selective Elimination of the γC Binding Epitope. J Biol Chem. 2010;285(16):12223-12231. doi:10.1074/jbc.M110.101444
CrossRef - Alsedfy MY, Ebnalwaled AA, Moustafa M, Said AH. Investigating the binding affinity, molecular dynamics, and ADMET properties of curcumin-IONPs as a mucoadhesive bioavailable oral treatment for iron deficiency anemia. Sci Rep. 2024;14(1):22027. doi:10.1038/s41598-024-72577-8
CrossRef - Lin M, Guo J tao. New insights into protein–DNA binding specificity from hydrogen bond based comparative study. Nucleic Acids Res. 2019;47(21):11103-11113. doi:10.1093/nar/gkz963
CrossRef - Lightfoot YL, Selle K, Yang T, et al. SIGNR 3‐dependent immune regulation by Lactobacillus acidophilus surface layer protein A in colitis. EMBO J. 2015;34(7):881-895. doi:10.15252/embj.201490296
CrossRef - Stolfi C, Rizzo A, Franzè E, et al. Involvement of interleukin-21 in the regulation of colitis-associated colon cancer. J Exp Med. 2011;208(11):2279-2290. doi:10.1084/jem.20111106
CrossRef - McGeachy MJ, Chen Y, Tato CM, et al. The interleukin 23 receptor is essential for the terminal differentiation of interleukin 17–producing effector T helper cells in vivo. Nat Immunol. 2009;10(3):314-324. doi:10.1038/ni.1698
CrossRef - Potestio L, Martora F, Lauletta G, Vallone Y, Battista T, Megna M. The Role of Interleukin 23/17 Axis in Psoriasis Management: A Comprehensive Review of Clinical Trials. Clin Cosmet Investig Dermatol. 2024;Volume 17:829-842. doi:10.2147/CCID.S462797
CrossRef - Sagmeister T, Gubensäk N, Buhlheller C, et al. The molecular architecture of Lactobacillus S-layer: Assembly and attachment to teichoic acids. Proc Natl Acad Sci. 2024;121(24):e2401686121. doi:10.1073/pnas.2401686121
CrossRef - Todorov SD. Bacteriocins from Lactobacillus plantarum production, genetic organization and mode of action: produção, organização genética e modo de ação. Braz J Microbiol. 2009;40(2):209-221. doi:10.1590/S1517-83822009000200001
CrossRef - C S, S. DK, Ragunathan V, Tiwari P, A. S, P BD. Molecular docking, validation, dynamics simulations, and pharmacokinetic prediction of natural compounds against the SARS-CoV-2 main-protease. J Biomol Struct Dyn. 2022;40(2):585-611. doi:10.1080/07391102.2020.1815584
CrossRef - Pantsar T, Poso A. Binding Affinity via Docking: Fact and Fiction. Molecules. 2018;23(8):1899. doi:10.3390/molecules23081899
CrossRef - Moll GN, Van Den Akker E, Hauge HH, et al. Complementary and Overlapping Selectivity of the Two-Peptide Bacteriocins Plantaricin EF and JK. J Bacteriol. 1999;181(16):4848-4852. doi:10.1128/JB.181.16.4848-4852.1999
CrossRef - Hertati A, Hayashi S, Ogawa Y, Yamamoto T, Kadowaki M. Interleukin-4 Receptor α Subunit Deficiency Alleviates Murine Intestinal Inflammation In Vivo Through the Enhancement of Intestinal Mucosal Barrier Function. Front Pharmacol. 2020;11:573470. doi:10.3389/fphar.2020.573470
CrossRef - Hammer GE, Ma A. Molecular Control of Steady-State Dendritic Cell Maturation and Immune Homeostasis. Annu Rev Immunol. 2013;31(1):743-791. doi:10.1146/annurev-immunol-020711-074929
CrossRef - Anderssen EL, Diep DB, Nes IF, Eijsink VGH, Nissen-Meyer J. Antagonistic Activity of Lactobacillus plantarum C11: Two New Two-Peptide Bacteriocins, Plantaricins EF and JK, and the Induction Factor Plantaricin A. Appl Environ Microbiol. 1998;64(6):2269-2272. doi:10.1128/AEM.64.6.2269-2272.1998
CrossRef - Ramírez D, Caballero J. Is It Reliable to Take the Molecular Docking Top Scoring Position as the Best Solution without Considering Available Structural Data? Molecules. 2018;23(5):1038. doi:10.3390/molecules23051038
CrossRef - Kageyama Y, Nishizaki Y, Aida K, et al. Lactobacillus plantarum induces innate cytokine responses that potentially provide a protective benefit against COVID‑19: A single‑arm, double‑blind, prospective trial combined with an in vitro cytokine response assay. Exp Ther Med. 2021;23(1):20. doi:10.3892/etm.2021.10942
CrossRef - Terefe EM, Ghosh A. Molecular Docking, Validation, Dynamics Simulations, and Pharmacokinetic Prediction of Phytochemicals Isolated From Croton dichogamus Against the HIV-1 Reverse Transcriptase. Bioinforma Biol Insights. 2022;16:11779322221125605. doi:10.1177/11779322221125605
CrossRef - Yan Y, Zhang D, Zhou P, Li B, Huang SY. HDOCK: a web server for protein–protein and protein–DNA/RNA docking based on a hybrid strategy. Nucleic Acids Res. 2017;45(W1):W365-W373. doi:10.1093/nar/gkx407
CrossRef - Yu W, MacKerell AD. Computer-Aided Drug Design Methods. In: Sass P, ed. Antibiotics. Vol 1520. Methods in Molecular Biology. Springer New York; 2017:85-106. doi:10.1007/978-1-4939-6634-9_5
CrossRef
Accepted on: 22-06-2026
Second Review by: Dr. Ana Golez
Final Approval by: Dr. Achyut Shankar